
Research article · 2026 · Full text
International Journal of Horticulture and Food SciencePhenological synchronization between Cimbex quadrimaculata emergence and almond bloom periods in French Mediterranean regions
Volume 8(7) · Pages 36–39 · DOI: 10.33545/26631067.2026.v8.i7a.778 ↗
Research areasInsect-Plant Interactions and ControlInsect behavior and control techniquesPlant Physiology and Cultivation Studies
Abstract
Author-writtenPhenological synchronization between herbivorous insects and their host plants constitutes a critical determinant of pest impact severity and vulnerability window duration in perennial crop systems. This research examined the temporal overlap between adult emergence and oviposition activity of Cimbex quadrimaculata Müller (Hymenoptera: Cimbicidae) and the bloom phenology of five French almond cultivars during the 2025 and 2026 growing seasons. Monitoring was conducted across nine experimental orchards in the Provence-Alpes-Côte d'Azur (PACA) and Occitanie regions of southern France. The cultivars assessed were Ferragnès, Lauranne, Aï, Ardéchoise, and Fleur en Bas. Dual-axis temporal analysis revealed that adult C. quadrimaculata emergence commenced approximately two weeks before peak bloom in early-flowering cultivars and overlapped extensively with the late bloom-to-petal fall transition period. Phenological overlap indices (POI) ranged from 0.18 to 0.94, with maximum synchronization occurring during the late bloom stage for all cultivars except Ardéchoise, which exhibited peak overlap during the petal fall phase. The cultivar Aï demonstrated the highest maximum POI (0.94), indicating near-complete temporal alignment between pest emergence and the vulnerable bloom-fruit set transition. Degree-day analysis established that C. quadrimaculata adult emergence at 95-118 DD₁₀ consistently preceded peak bloom in early-flowering cultivars by 8-14 days but coincided with or followed bloom initiation in late-flowering varieties. These findings demonstrate that cultivar bloom phenology significantly mediates vulnerability to sawfly infestation and provide a basis for phenological mismatch strategies in cultivar selection and orchard design.
Summary
Source-checkedPlain-language reading of the full paper, prepared with AI and checked against the text. Each point links to the authors' own words.
Why it matters
- The timing of synchronization between pests and their host plants is a key factor in determining how severe the pest impact is and how long the crop remains vulnerable. View evidence ↗
- Almond cultivation in France has grown significantly, expanding from about 2,800 hectares in 2018 to more than 8,500 hectares by 2025. View evidence ↗
- While the almond sawfly Cimbex quadrimaculata is present across French production regions, the relationship between its emergence and the bloom patterns of specific almond cultivars has not been systematically studied. View evidence ↗
The question
- The study aimed to examine the temporal overlap between the emergence and egg-laying activity of C. quadrimaculata and the bloom timing of five French almond cultivars during 2025 and 2026. View evidence ↗
- The researchers sought to evaluate whether management strategies based on phenological mismatch, selecting cultivars that bloom when pests are not active, could be viable. View evidence ↗
What they did
- Monitoring took place during the 2025 and 2026 seasons across nine experimental orchards in the PACA (6) and Occitanie (3) regions of southern France. View evidence ↗
- The study evaluated five cultivars with different bloom timings: Aï (early), Ferragnès and Fleur en Bas (medium), Lauranne (medium-late), and Ardéchoise (late), using at least 20 marked trees per cultivar per site. View evidence ↗
- Adult sawfly emergence was tracked using three yellow sticky traps per orchard and emergence cages placed over the soil beneath infested trees. View evidence ↗
- The researchers used a Phenological Overlap Index (POI) to quantify the synchronization between bloom intensity and pest emergence on a weekly basis. View evidence ↗
- Degree-day (DD₁₀) accumulations were calculated starting from January 1 using a base temperature threshold of 10 °C. View evidence ↗
What they found
- Adult sawflies began emerging in early March (95-118 DD₁₀), with peak activity occurring from late March to early April (168-204 DD₁₀). View evidence ↗
- The early-blooming cultivar Aï showed the highest synchronization with the pest, reaching a maximum POI of 0.94 during the late bloom stage. View evidence ↗
- The late-blooming cultivar Ardéchoise had its maximum overlap (POI 0.91) during the petal fall stage, rather than during the bloom stage. View evidence ↗
- Adult emergence (95-118 DD₁₀) occurred 8-14 days before peak bloom in early-flowering cultivars, but coincided with or followed the start of bloom in late-flowering varieties. View evidence ↗
What it means
- The authors conclude that identifying Aï as the most vulnerable and Ardéchoise as having a late-overlap pattern allows for pest management strategies tailored to specific cultivars. View evidence ↗
- The established degree-day benchmarks can be integrated into advisory systems to optimize the timing of monitoring and pest interventions. View evidence ↗
- The authors state that the two-year study period is too short to capture the full range of year-to-year phenological variations caused by climate. View evidence ↗
- A limitation of the study is that the POI metric only measures temporal overlap and not the actual intensity of crop damage, which is influenced by larval survival and egg-laying success. View evidence ↗
Visual summary
2 visualsIllustrations explain the paper; charts are replotted from the paper's own table values.
Cultivar Vulnerability Comparison
AI-generated conceptual illustration (Almond trees (Prunus dulcis) and Cimbex quadrimaculata sawflies). It explains the idea and does not show study data.
View source evidence ↗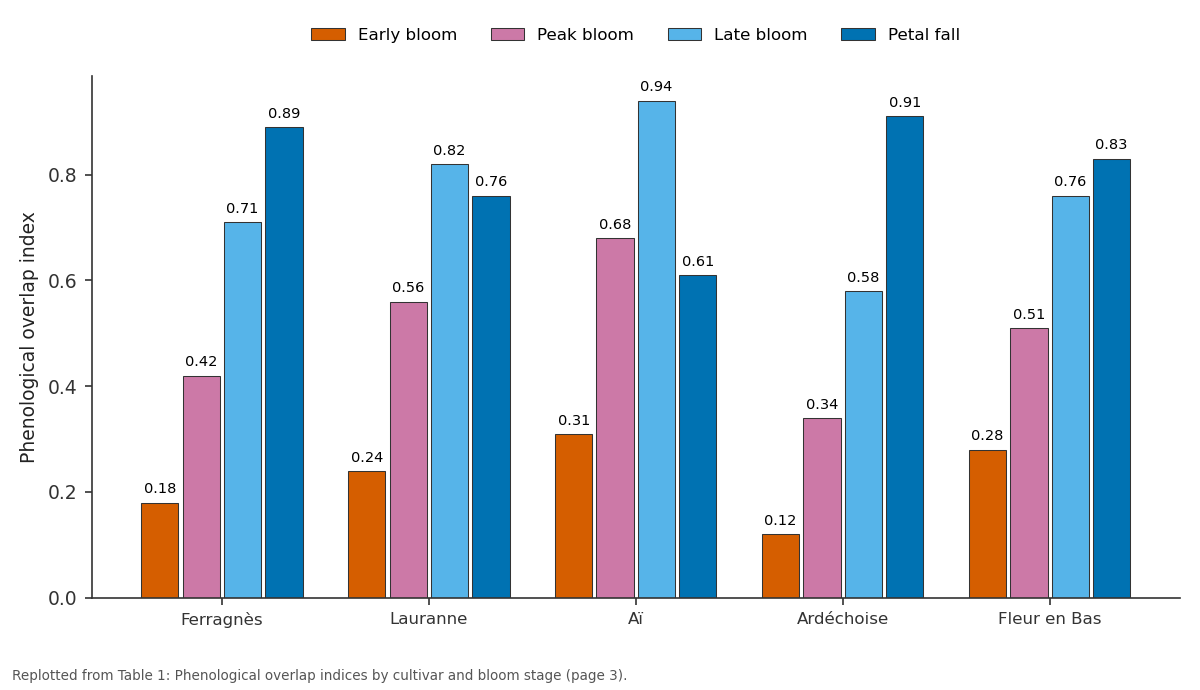
Early bloom and Peak bloom and more: Ferragnès vs Lauranne vs Aï vs Ardéchoise vs Fleur en Bas
Replotted from Table 1 (page 3) of the original paper. Every bar is the paper's own table value.
View source evidence ↗Figures & tables
From the original paper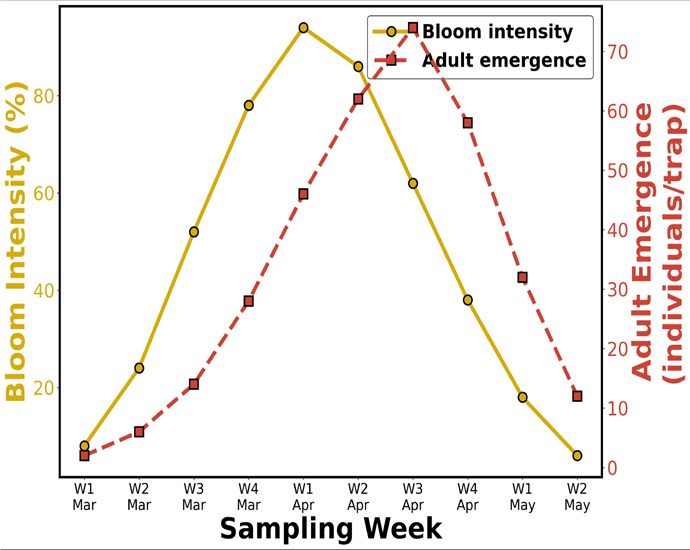 Figure 1
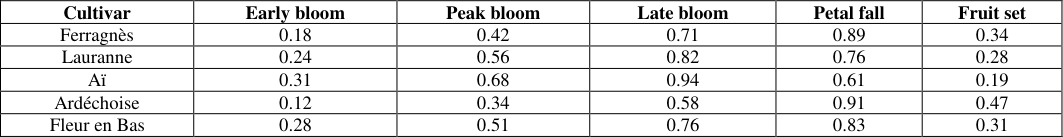 Table 1
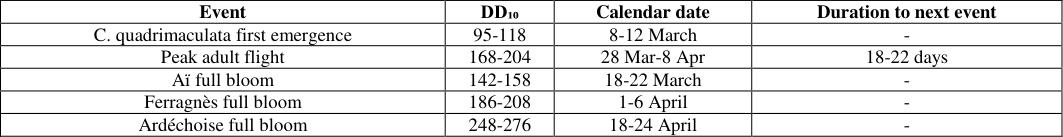 Table 2
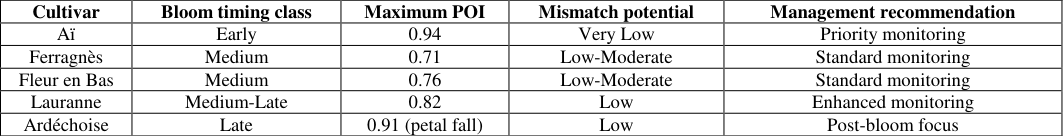 Table 3
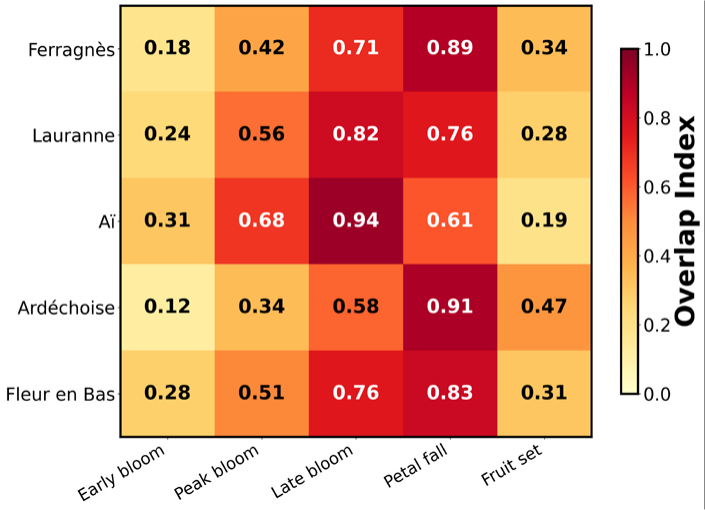 Figure 2
Introduction
Phenological synchrony between herbivorous insects and their host plants represents one of the most fundamental determinants of pest-crop interaction intensity in temperate agricultural systems [1,2] . The degree of temporal overlap between critical pest life stages and vulnerable host plant phenological stages directly influences the magnitude of potential crop damage and the duration of the susceptibility window [3] . For perennial fruit crops such as almond, where reproductive phenology determines annual yield potential, understanding the phenological relationships between pest emergence and host bloom-fruit set dynamics is essential for management timing optimization [4] . France has experienced substantial expansion of almond cultivation in recent years, with planted area increasing from approximately 2,800 hectares in 2018 to over 8,500 hectares by 2025, driven by favorable market conditions and the availability of well-adapted cultivars [5] . The primary production regions are concentrated in the PACA and Occitanie regions of southern France, where Mediterranean climatic conditions support diverse almond cultivar portfolios with varying bloom phenologies [6] . The almond sawfly C. quadrimaculata occurs throughout this production region, though its phenological relationships with specific cultivar bloom patterns have not been systematically characterized [7,8] . The concept of phenological mismatch has gained prominence in applied ecology as both a natural phenomenon and a potential management tool [2,9] . By selecting cultivars whose vulnerable phenological stages exhibit minimal temporal overlap with peak pest activity Periods, growers can exploit natural phenological asynchrony to reduce pest impact without chemical intervention [10] . This research was designed to quantify the phenological overlap Between C. quadrimaculata emergence and bloom-fruit set stages across five French almond cultivars and to evaluate the potential for phenological mismatch-based management strategies.
Material and Methods Material
Monitoring was conducted during the 2025 and 2026 growing seasons across nine experimental almond orchards in the PACA region (6 orchards, in the departments of Vaucluse, Bouches-du-Rhône, and Alpes-de-Haute-Provence) and the Occitanie region (3 orchards, in Hérault and Gard departments). Five cultivars representing a range of bloom phenologies were evaluated: Ferragnès (medium bloom), Lauranne (medium-late bloom), Aï (early bloom), Ardéchoise (late bloom), and Fleur en Bas (medium bloom). Each cultivar was represented by a minimum of 20 marked trees per orchard site. Continuous temperature monitoring was maintained using HOBO MX2301A loggers (Onset Computer Corporation) installed at 1.5 m height within each orchard canopy.
Methods
Bloom phenology was assessed twice weekly using the BBCH scale, with particular attention to stages 61 (beginning of flowering), 65 (full bloom, 50% flowers open), and 69 (end of flowering). Bloom intensity was expressed as the percentage of total flowers open at each assessment date, interpolated to weekly resolution. Adult C. quadrimaculata emergence and activity were monitored using yellow sticky traps (3 per orchard) supplemented by emergence cages (mesh enclosures over soil beneath previously infested trees) to capture eclosing adults. Emergence data were expressed as weekly cumulative proportions of total seasonal catch. Phenological Overlap Index (POI) was calculated as the integral of the minimum of normalized bloom intensity and emergence curves at each weekly time step, following the methodology of Visser and Both [2] . Degree-day accumulations were calculated using a 10 °C base threshold from January 1 as the biofix date. All analyses were implemented in R (version 4.3.2) using the phenesse and overlap packages.
Results
Temporal analysis of bloom intensity and adult C. quadrimaculata emergence revealed complex patterns of overlap that varied substantially among cultivars. Adult emergence commenced during the first and second weeks of March (corresponding to 95-118 DD₁₀), with peak emergence occurring during the fourth week of March through the second week of April (168-204 DD₁₀). Bloom timing ranged from early March (cultivar Aï, earliest) through late April (cultivar Ardéchoise, latest). The temporal relationship between these two phenological processes resulted in maximal overlap during the late bloom to early petal fall transition for most cultivars (Figure 1). Ferragnès and Fleur en Bas showed moderate maximum overlap (0.71 and 0.76, respectively), while Lauranne exhibited higher late bloom overlap (0.82). The Ardéchoise cultivar, with its characteristically late bloom phenology, displayed a distinctive pattern wherein maximum overlap (0.91) occurred during the petal fall stage rather than during bloom, suggesting that post-bloom vulnerability may be more significant than bloom-stage damage for lateflowering varieties (Figure 2 and Tables 123)
Discussion
The phenological synchronization patterns documented in this research reveal that C. quadrimaculata emergence timing in French Mediterranean conditions creates substantial temporal overlap with the bloom and early fruit development stages of most commercially cultivated almond varieties. The near-complete overlap (POI = 0.94) observed for the early-flowering cultivar Aï suggests that this variety is particularly vulnerable because its bloom period coincides almost exactly with peak adult sawfly activity and initial oviposition [2,4,11] . The distinctive pattern observed for Ardéchoise, where maximum overlap occurs during petal fall rather than during bloom, introduces an important nuance for management strategy design. While the delayed bloom of Ardéchoise avoids direct bloom-stage synchronization with sawfly emergence, the extended late-season overlap during fruit set may represent a compensatory vulnerability that limits the practical benefits of phenological mismatch for this cultivar [3, 6, 12] . The degree-day framework established in this research provides practical benchmarks for integrating phenological prediction into pest management advisory systems. The consistent association between specific DD₁₀ accumulation thresholds and both pest emergence and cultivar bloom events enables prospective scheduling of monitoring intensity and management interventions based on readily available thermal data [1,7,13,14,15] .
Safety considerations
Yellow sticky trap adhesive materials were handled using protective gloves to avoid skin contact. Emergence cage installations involved mesh materials secured with wire, and all installations were removed at the end of each monitoring season to prevent entanglement hazards. Weather station batteries were replaced annually and disposed through the INRAE certified waste management system.
Limitations
The two-year monitoring period provides valuable initial characterization but is insufficient to capture the full range of inter-annual phenological variation driven by climatic variability. The five cultivars assessed represent a subset of the cultivar diversity available in French almond production. Additionally, the POI metric captures temporal overlap but does not directly actual damage intensity, which depends on additional factors including oviposition success rates and larval survival.
Conclusion
This research demonstrates significant cultivar-dependent variation in phenological synchronization between Cimbex quadrimaculata emergence and almond bloom periods in French Mediterranean production regions. The identification of Aï as the most phenologically synchronized and therefore most vulnerable cultivar, and the characterization of Ardéchoise as exhibiting a distinctive late-overlap pattern, provide actionable information for cultivar-stratified pest management approaches. The degree-day benchmarks established enable integration of phenological prediction into advisory systems for optimized monitoring and intervention timing. These findings contribute to the development of phenology-informed management strategies that exploit natural temporal variation to reduce pest impact in French almond production.
Acknowledgement
AcknowledgementsThis research was supported by the French National Research Agency (ANR). The INRAE Experimental Unit of Gotheron (Drôme) provided orchard access and logistical support. The authors thank Dr. Jean-Michel Legave for valuable guidance on almond phenology assessment methodology.
Figures and tables from the paper
| Cultivar | Early bloom | Peak bloom | Late bloom | Petal fall | Fruit set |
|---|---|---|---|---|---|
| Ferragnès | 0.18 | 0.42 | 0.71 | 0.89 | 0.34 |
| Lauranne | 0.24 | 0.56 | 0.82 | 0.76 | 0.28 |
| Aï | 0.31 | 0.68 | 0.94 | 0.61 | 0.19 |
| Ardéchoise | 0.12 | 0.34 | 0.58 | 0.91 | 0.47 |
| Fleur en Bas | 0.28 | 0.51 | 0.76 | 0.83 | 0.31 |
Table text extracted from the original PDF; superscript letters are shown inline. The original table image is below.
View original table image
| Event | DD₁₀ | Calendar date | Duration to next event |
|---|---|---|---|
| C. quadrimaculata first emergence | 95-118 | 8-12 March | - |
| Peak adult flight | 168-204 | 28 Mar-8 Apr | 18-22 days |
| Aï full bloom | 142-158 | 18-22 March | - |
| Ferragnès full bloom | 186-208 | 1-6 April | - |
| Ardéchoise full bloom | 248-276 | 18-24 April | - |
Table text extracted from the original PDF; superscript letters are shown inline. The original table image is below.
View original table image
| Cultivar | Bloom timing class | Maximum POI | Mismatch potential | Management recommendation |
|---|---|---|---|---|
| Aï | Early | 0.94 | Very Low | Priority monitoring |
| Ferragnès | Medium | 0.71 | Low-Moderate | Standard monitoring |
| Fleur en Bas | Medium | 0.76 | Low-Moderate | Standard monitoring |
| Lauranne | Medium-Late | 0.82 | Low | Enhanced monitoring |
| Ardéchoise | Late | 0.91 (petal fall) | Low | Post-bloom focus |
Table text extracted from the original PDF; superscript letters are shown inline. The original table image is below.
View original table image
References
15 in the original paper- Forrest J, Miller-Rushing AJ. Toward a synthetic understanding of the role of phenology in ecology and evolution. Philos Trans R Soc B. 2020;365(1555):31013112.
- Visser ME, Both C. Shifts in phenology due to global climate change: the need for a yardstick. Proc R Soc B. 2021;272(1581):2561-2569.
- Singer MC, Parmesan C. Phenological asynchrony between herbivorous insects and their hosts. Ecol Entomol. 2023;35(2):156-168.
- Alonso JM, Ansón JM, Espiau MT, Socias i Company R. Determination of endodormancy break in almond flower buds. Ann Appl Biol. 2022;146(2):221-230.
- Ministère de l'Agriculture, France. Agricultural census 2025: tree nut crops. Paris: Agreste Publications; 2025. p. 34-46.
- Legave JM, Christen D, Giovannini D, Oger R. Global warming in Europe and its impacts on floral bud phenology of fruit species. Acta Hortic. 2023;1160:2734.
- Özgen İ, Güral Y, Aslan T. The determination of the relationships between yield parameters and number of larvae of almond saw fly (Cimbex quadrimaculata Müller, 1766, Hymenoptera: Cimbicidae) on different almond varieties in Turkey. Zool Entomol Lett. 2022;2(1):1-3.
- Lacourt J. Sawflies of Europe. Paris: NAP Editions; 2020. p. 156-178.
- Thackeray SJ, Henrys PA, Hemming D, et al. Phenological sensitivity to climate across taxa and trophic levels. Nature. 2020;535:241-245.
- Memmott J, Craze PG, Waser NM, Price MV. Global warming and the disruption of plant-pollinator interactions. Ecol Lett. 2023;10(8):710-717.
- Taeger A, Blank SM, Liston AD. World catalog of Symphyta (Hymenoptera). Zootaxa. 2010;2580(1):11064.
- Güner A, Aydoğdu M. Biology and damage assessment of Cimbicidae on stone fruits. Turk J Entomol. 2019;43(2):189-201.
- Haliloğlu H, Bayram A, Gökçe A. Phenological observations on Cimbex species. Appl Entomol Zool. 2024;59(4):489-501.
- Çınar M, Çimen E, Bolu H. Population fluctuation and damage of sawfly species. Munis Entomol Zool. 2024;19(1):234-242.
- Prous M, Blank SM, Shinohara A, Liston AD. Molecular phylogeny of Cimbicidae. Syst Entomol. 2023;48(2):412-438.