
Research article · 2019 · Full text
International Journal of Horticulture and Food ScienceInfluence of macronutrient acumulation of “Magnum” watermelon by phosphate doses and aplication maners in calcareous soil
Volume 1(2) · Pages 27–34 · DOI: 10.33545/26631067.2019.v1.i2a.26 ↗
Research areasGrowth and nutrition in plantsIrrigation Practices and Water ManagementPlant nutrient uptake and metabolism
Abstract
Author-writtenInformation on the nutritional need of the watermelon crop is required particularly for P, due to the dynamics of this element in the soil and its low availability in many soils in the semi-arid region. The objective of this work was to evaluate the biomass production and the macronutrient extraction of the cv. Magnum irrigated under the influence of phosphate fertilization. The experiment was carried out in a medium textured Cambisol in Upanema, state of Rio Grande do Norte, in a randomized block experiment design, using the split-plot factorial scheme with four replications. The treatments consisted of 76, 168, 275 and 397 kg ha-1 of P2O5, which were applied in two manners: F0 – 100% in pre-planting and F1 – in pre-planting + fertirrigation (50 kg ha- 1 as MAP). Two additional treatments were also applied: Adc1 – no phosphate; and Adc2 – with phosphate only in fertirrigation. Fertilization F1 provided greater accumulations of P and S, but, in general, the effects of the doses were dependent on the fertilization system, especially the treatments F0275 and F1168 regarding the accumulation of other nutrients.
Summary
Source-checkedPlain-language reading of the full paper, prepared with AI and checked against the text. Each point links to the authors' own words.
Why it matters
- Understanding the phosphorus (P) needs of watermelon is critical because P has low availability in many semi-arid region soils. View evidence ↗
- Phosphorus is often a limiting nutrient in calcareous soils because higher pH levels and the precipitation of calcium and magnesium reduce its solubility. View evidence ↗
- To combat low phosphorus mobility and soil adsorption, it is generally recommended to apply phosphate fertilizers in a localized manner. View evidence ↗
The question
- The study aimed to evaluate how phosphate fertilization affects biomass production and macronutrient extraction in 'Magnum' watermelon. View evidence ↗
What they did
- The experiment took place from September to November 2013 in a calcareous Cambisol soil in Upanema, Rio Grande do Norte. View evidence ↗
- Four doses of P2O5 (76, 168, 275, and 397 kg ha-1) were tested using two application methods: 100% pre-planting (F0) or a combination of pre-planting and fertirrigation (F1). View evidence ↗
- The study included two control treatments: one with no phosphate (Adc1) and one with phosphate applied only via fertirrigation (Adc2). View evidence ↗
- Plants were sampled at 28, 38, 54, and 69 days after emergence (DAE), then divided into stem, leaves, and fruits for weighing and drying at 65 °C. View evidence ↗
What they found
- At 69 DAE, nitrogen (N) accumulation was highest in the F0275 treatment (20.36 g plant-1) and lowest in the F1397 treatment (13.20 g plant-1). View evidence ↗
- The combined pre-planting and fertirrigation method (F1) resulted in higher phosphorus (P) accumulation than the pre-planting only method (F0), with a difference of 0.81 g plant-1 at 69 DAE. View evidence ↗
- Maximum P accumulation varied from 1.32 to 2.84 g plant-1, driven by both the fertilization method (0.81 g plant-1 difference) and the dose (0.71 g plant-1 difference between 397 and 76 kg ha-1). View evidence ↗
- Calcium (Ca) accumulation was highest at the highest phosphate doses, with F1397 reaching 20.32 g plant-1 and F0397 reaching 14.36 g plant-1. View evidence ↗
- Without phosphate (Adc1), maximum Ca accumulation was only 6.62 g plant-1, which is 32% to 64% of the values seen in other treatments. View evidence ↗
- The highest magnesium (Mg) accumulation was found in F1397 (2.58 g plant-1 at 52 DAE), followed by F0275, F0397, and F1168. View evidence ↗
- Sulfur (S) accumulation was higher in the F1 method (0.88 to 1.12 g plant-1) compared to the F0 method (0.71 to 0.90 g plant-1) across the tested phosphate doses. View evidence ↗
What it means
- The authors concluded that while F1 fertilization maximizes P and S accumulation, the accumulation of other nutrients depends on the interaction between the dose and the application method, with F0275 and F1168 being particularly effective. View evidence ↗
Visual summary
1 visualsIllustrations explain the paper; they do not show study data.
Fertilization Treatment Scheme
AI-generated conceptual illustration (Magnum watermelon plants in calcareous soil). It explains the idea and does not show study data.
View source evidence ↗Figures & tables
From the original paper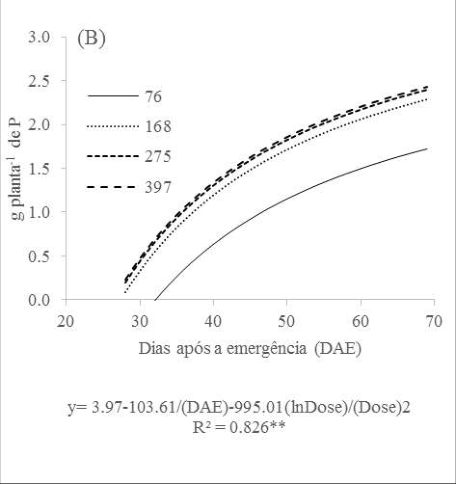 Figure 2
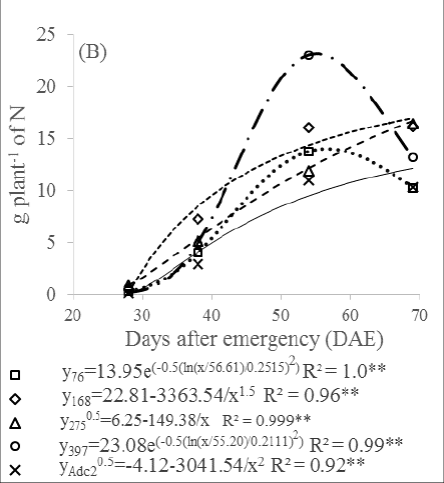 Figure 1
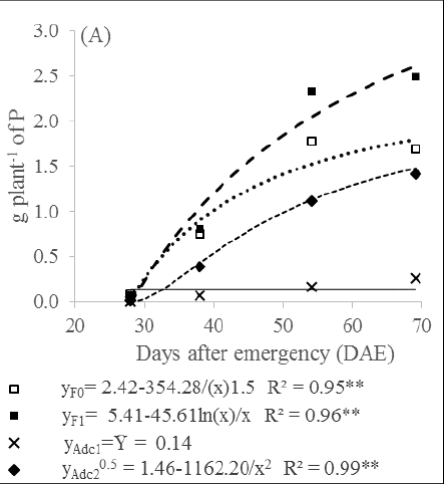 Figure 2
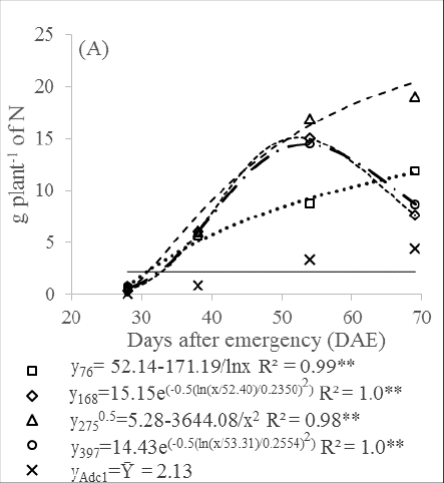 Figure 1
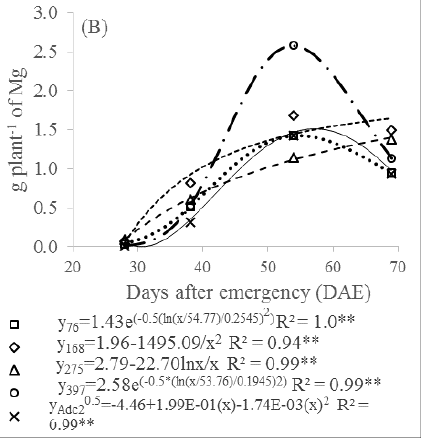 Figure 5
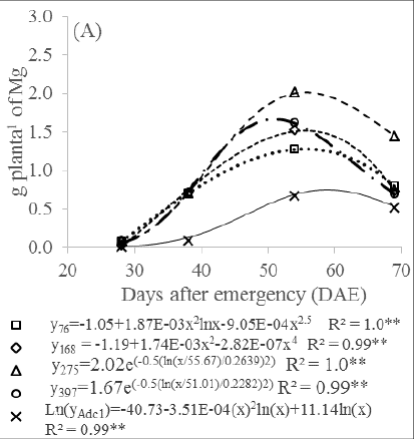 Figure 5
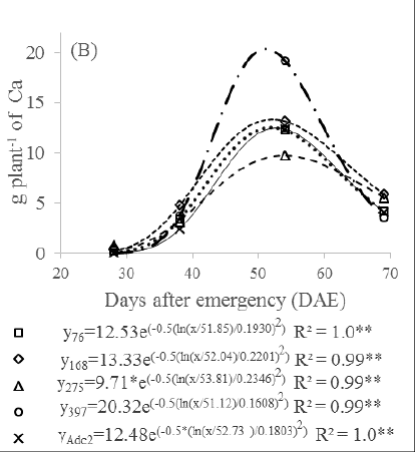 Figure 4
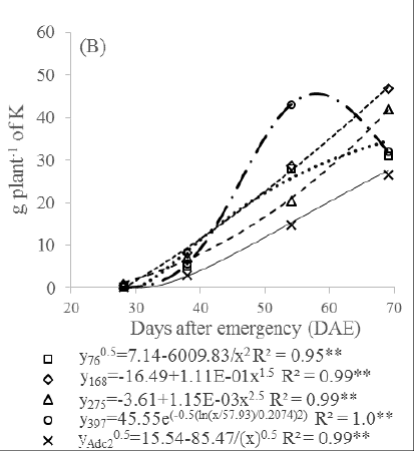 Figure 3
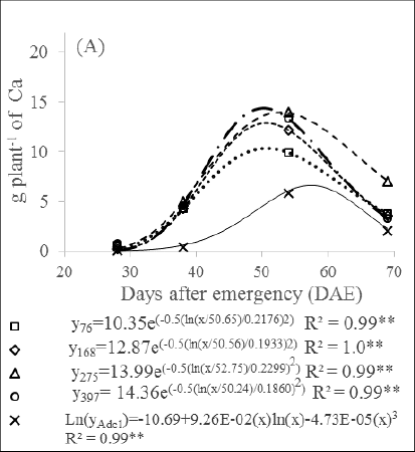 Figure 4
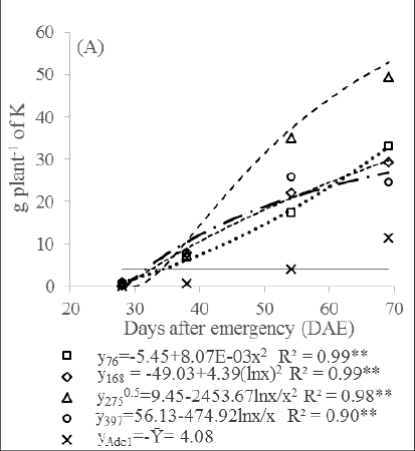 Figure 3
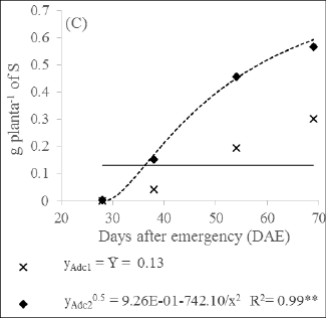 Figure 6
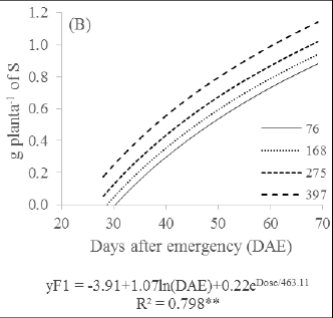 Figure 6
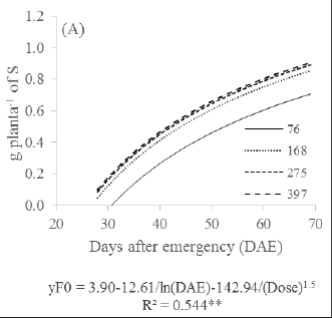 Figure 6
Introduction
Plant growth and nutrient uptake patterns are essential in crop nutrition and fertilization, especially for short-cycle crops such as watermelon, therefore meeting the plant demand over periods of the greatest demand (ALMEIDA et al., 2014) [1] . However, the absorption and proportion between nutrients depend on both the cultivar and external factors that influence the process. According to Fernandes and Soratto (2012) [7] several studies have shown that the nutritional level of phosphorus (P) may affect the absorption of other nutrients and consequently, the nutrition and production of the crops. Despite that, many studies consider only the ontogenetic variations in the absorption and utilization of the nutrients by the crop, neglecting the effects resulting from its nutritional management. In the watermelon crop, source-drain relations undergo major changes after pollination, since the fruits are the favored drains in relation to the vegetative organs (LINS et al., 2013) [12] . Under these conditions, mineral nutrients gain importance as productivity limiting factors, particularly when associated with a decline in the uptake by the roots (MARSCHNER, 2012) [15] . In general, P has been considered one of the most limiting nutrients, even in calcareous soils (MOHAMMAD et al., 2004) [17] due to the reduced solubility of P compounds at higher pH and Ca and Mg precipitations (HOPKINS et al., 2014) [10] . Silva et al. (2012) [22] explain that the absorption of P by the watermelon crop is small because of its low mobility in the soil and the great proportion that is adsorbed to the colloids. To reduce this effect, the general recommendation is to apply the total dose of phosphate in a localized way, in order to reduce contact with the soil. For Mohammad et al. (2004) [17] the conventional application of P in pre-planting has the advantage of providing high concentrations in the soil solution at the initial stages of the crops, but a continuous supply of P through irrigation water (fertirrigation) may increase its absorption at the end of the production cycle, especially for crops with narrower root volume. Barreto and Fernandes (2002) [5] hypothesized that the mixture of phosphate fertilizer with higher soil fractions could in some cases increase the efficiency of use of phosphate fertilizer, especially in soils with low clay and iron and aluminum oxide contents, in contrast to typical tropical acid soils.
Thus, the objective of this work was to evaluate the macronutrient extraction of the cv. Magnum watermelon in calcareous soils under the influence of phosphate fertilization management.
Material and Methods
This study was conducted from September to November 2013 in a Cambisol of calcareous origin of the Jandaíra formation, in the municipality of Upanema, state of Rio Grande do Norte, (5°35´04'' S, 37°12'08'' W and 122 m above sea level). The predominant climate in the region is hot and dry -BSwh' type, according to the climatic classification of Köppen. Over the experimental period, the average daily air temperature ranged between 26.9 and 28.2 °C and the relative humidity of the air was 65% (data from the automatic station of Mossoró A318 -INMET). Before the installation of the experiment, the 0-20 cm layer was sampled for physicochemical characterization (Table 1). An initial sampling of the 0-20 cm layer was carried out for chemical characterization according to Silva (2009) [21] showing the following values: pH (H2O) = 7.4; organic matter (in g kg -1 ) = 23.86; P Mehlich (in mg dm -3 ) = 4; K + , Na + , Ca 2+, Mg 2+ , Al 3+ and H + Al 3+ (in mmolc dm -3 ) and V (%) = 5.60; 0.70; 48.4; 21.1; 0.0; 14.9 and 84. The contents of Cu, Fe, Mn, and Zn were extracted using DTPA solution pH 7.3, which was 0.8, 0.7, 17.9 and 7 mg dm -3 , respectively and 24 mg L -1 for the remaining P dosage obtained in 0.01 M CaCl2 solution using 60 mg L -¹ of P of initial concentration in the 1:10 soil: solution ratio. The granulometric analysis indicated 228.87 and 685 g kg -1 of clay, silt, and sand, respectively, in which the clay fraction was obtained by the pipette method; silt by the difference of mass between the total sample and the sand by sieving. The water used in the irrigations had the following chemical characteristics: pH = 7.8; EC = 0.47 dS m -1 ; Ca 2+ = 2.25; Mg 2+ = 0.89; K + = 0.44; Na + =2.16; Cl -= 1.31; HCO3 -= 4.00; CO3 2-= 0.16 (mmolc L -1 ). The experiment was conducted in a complete randomized block design, in a factorial scheme (2 x 4 + 2) x 4, with two forms of fertilization management and four doses of P and two additional treatments using subdivided plots, corresponding to four periods. Phosphate fertilization forms consisted of pre-planting application (F0) and pre-planting + topdressing (F1) of four P2O5 (76, 168, 275 and 397 kg ha -1 ) doses. The pre-planting doses were hand applied using triple superphosphate (TSP) (41% P2O5), while the topdressing fertilization was carried out via irrigation water (fertirrigation) using monoammonium phosphate (MAP) (60% P2O5). Two additional treatments were also applied. Those treatments were the lack of P application (Adc1) and application of P only in topdressing 50 kg ha -1 P2O5 (Adc2). The soil was previously tilled by means of plowing and harrowing, rising mounds of 0.30 m in height and 0.60 m in width. The area of the experimental plots was 27.36 m² (14.4 mx 1.9 m), with a useful plot of 13.68 m² (7.2 mx 1.9 m), containing a total of eight plants spaced by 0.90 x 1.9 m. The 'Magnum' watermelon seedlings were produced in expanded polystyrene trays with 200 cells filled with Plantimax commercial farming substrate and coconut fiber. When the seedlings displayed two definitive leaves, they were transplanted to the area, seven days after emergence (DAE) or twelve days after sowing (DAS), on September 28, 2013. Irrigation was performed daily through a drip system, with emitters spaced at 0.30 m. The irrigation system was evaluated three times over cultivation, according to Merrian and Keller (1978) [16] with the average flow and emission uniformity coefficients of 1.20 L h -1 and 93.2%, respectively. Irrigation management was carried out by monitoring the soil moisture with the aid of tensiometers, in order to maintain soil with matrix potential higher than -30 kPa. The fraction of the phosphate fertilization in pre-planting was hand applied in pits at each 0.30 m and next to each emitter. It was applied in all treatments 100 kg ha -1 Barimicro fertilizer (FTE BR12) containing 1.8% B; 0.8% Cu; 2.0% Mn; 9.0% Zn; and 4.0% of S. Nitrogen and potassium were applied via fertirrigation for all treatments, with totals estimated by the models developed by Paula et al. (2011) [18] . It was applied 140 and 100 kg ha -1 N and K2O, respectively, which were distributed from the week following transplanting. A further 7.6 kg ha -1 CaO was applied between the 3 rd and 4 th week after transplanting. The sources used were urea, ammonium sulfate, potassium chloride, potassium nitrate, and calcium nitrate. One plant was collected per plot at 28, 38, 54 and 69 DAE. The collected plant was divided into stem, leaves, and fruits, which were weighed, and the respective subsamples removed and taken to drying in a forced air circulation oven at 65 °C. After drying, they were weighed and the data used to deduction of the estimate of the total dry biomass. For the evaluation of nutrient concentrations, the dry matter was first milled in Willey-type mill for chemical analysis according to Malavolta et al. (1997) [13] . Nitrogen concentrations were determined by the Kjeldahl semi-micro method, K by flame emission photometry, Ca and Mg by atomic absorption spectrophotometry, S by turbidimetry and P by metavanadate colorimetry. The accumulations of nutrients were obtained from the product between the dry biomass and their respective concentration in the material. Data were submitted to analysis of variance, by the F test, at 5% of significance using the System for Analysis of Variance -SISVAR software, version 5.3 (FERREIRA, 2010) [8] and calculation worksheet. Afterward, regression analysis was performed and the models whose coefficients were significant by the test at 5% probability were selected, favoring those with a higher F and R² and that provided a simpler and more coherent explanation for biological behavior, using * and ** to indicate significance at 1% and 5% probability, respectively.
Results and Discussion
An increase was observed in the N accumulation rates until 44 DAE for most treatments, which can be explained by the stimulation of N accumulation in the vegetative organs, functioning as a nutrient reserve for the reproductive phase that is about to start, so that half of the total N is accumulated until 38-44 DAE (Figure 1A-1B). For F0275treatment, an increase from 0.42 to 0.79 g day -1 was found in the N accumulation rate per plant, between 28 and 42 DAE, and then, it reduced from there up to 0.20 g day -1 at the end of the cycle (Figure 5A). On the other hand, in the F1168 treatment, higher N accumulation rates were observed at 28 DAE (1.22 g day -1 ), which was reduced to 0.13 g day -1 at the end of the cycle (Figure 5B). A higher maximum point for N accumulation was observed in F1397, (23.08 g plant -1 at 55 DAE), corresponding to approximately 134.95 kg ha -1 N (Figure 5B), but it showed a significant reduction from that point, which can be explained by the loss of biomass (data not shown). The F0397 treatment presented a pattern similar to F1397, but with less pronounced curvature at the point of maximum (53 DAE). The same occurs for F0168 and F176, both with maximums at 57 DAE (Figure 5A-5B). This is more likely to have been caused by fruit abortion rather than leaf senescence since N can be easily remobilized from leaves. In a study with the 'Tide' hybrid, Grangeiro and Cecílio Filho (2004) [9] found positive increases in N accumulation until the end of the cycle but observed a reduction in the vegetative part that was explained by a strong translocation for fruit development. The authors also indicated that N was the second most absorbed nutrient, accumulating 138.8 kg ha -1 or 71 g plant -1 (1,960 plants ha -1 ). In this work, N accumulations at the end of the cycle (69 DAE) followed the following decreasing order: 20.36 (F0275), 16.94 (F1168), 16.66 (F1275) and 13.20 g plant -1 (F1397) or 119.04; 99.04; 97.41 and 77.18 kg ha -1 N (5.847 plants ha -1 ), respectively (Figure 5A-5B). Working with cv. Olimpia, Silva et al. (2012) [22] reported a maximum N accumulation at 69 days after sowing (DAS) of 77.5 kg ha -1 or 10.04 g plant -1 (7,716 plants ha -1 ), while Vidigal et al. (2009) [24] estimated 21.16 g plant -1 or 105.8 kg ha -1 N for cv. Crimson Sweet (at 89 DAS) with a density of 5,000 plants ha -1 . The highest maximum N accumulation in Adc2 (12.12 g plant-1) (Figure 5B) in relation to F076 (11.70 g plant -1 ) (Figure 5A) can be attributed to the synergistic effect between P and N, by the use of MAP in fertirrigation. Araújo and Machado (2006) [4] discuss the role of P on the general regulatory effects of N absorption and assimilation. Fernandes and Soratto (2012) [7] found increased N concentrations in potato plants as P supply was increased, even after the stabilization of production from a certain level of P in the nutrient solution (>8 mg L -1 ). When studying the effects of the partial P supply to the roots of corn grown in nutrient solution, Alves et al. (1999) [3] observed a reduction in the accumulation of N in the aerial part when it is supplied separately from the P, attributing this result to the low concentration of P in the root. Figure 2A shows a greater accumulation of P with F1 fertilization than F0, with a difference of 0.81 g plant -1 at 69 DAE, therefore accumulating 50% of the total at 41 and 38 DAE, respectively. However, the application of 50 kg ha -1 P2O5 only in the fertirrigation (Adc2) resulted in slower initial P absorption since 50% of the respective maximum accumulation occurs at 44 DAE. The application of all P in fertirrigation may result in nutrient deficiencies in the initial phase of the crop, as observed by Marouelli et al. (2015) [14] in a work with tomato. According to Mohammad et al. (2004) [17] different studies indicate that the P applied in pre-planting is available earlier to the plants, but its concentration in the soil solution declines over time due to the adsorption and precipitation reactions. In this respect, despite the known benefits of localized application of phosphate fertilizers, the entire root zone needs P, so that the combination of fertilizer application techniques can be favorable, particularly in soils with low to medium levels of P (HOPKINS et al. al., 2014) [10] .
Around 50% of P totals was accumulated between 36 and 42 DAE and between 40 and 45 DAE at doses of 76 to 397 kg ha -1 P2O5 in F0 and F1 fertilizations, respectively (Figure 2A-2B). This is the result of the effects of localized phosphate fertilization on the initial availability of P, as already discussed since the increases in the doses for both fertilizations are due to pre-planting phosphate increments. Overall, the rapid observed accumulation of nutrients should be related to the experimental conditions, coinciding with the period in which 50% of the maximum accumulations occur for total biomass: between 37 and 46 DAE and between 41 and 47 DAE for the F0 and F1 treatments, respectively (data not shown) The total variation in the P maximum accumulation in the factorial treatments is from 1.32 to 2.84 g plant -1 (7.72 to 16.61 kg ha -1 ), which is attributable to the differences between F1 and F0 fertilizations (0.81 g plant -1 ) (Figure 2A) and between the doses of 397 and 76 kg ha -1 P2O5 (0.71 g plant -1 ) (Figure 2B). The accumulation of P in Adc2 (1.48 g plant -1 ) is equivalent to the 89 kg ha -1 dose of P2O5 in F0 fertilization. In work with cv. Magnum in sandy soil (8,333 plants ha -1 ), Pereira et al. (2018) [19] also observed effects of phosphate fertilization on P accumulation, indicating an increase of 0.29 g plant -1 when using the pre-planting + topdressing combination (0.96 g plant -1 ), in relation to fertilization in pre-planting (0.67 g plant -1 ), for a dose of 137 kg ha -1 P2O5. The authors explained that the combination of application forms was most likely to have contributed to the increase in P availability in the soil. It is worth noting that the effects on nutrient accumulation observed in the present work are derived from the combination of fertilization techniques rather than from the isolated application of P. Moreover, although some authors have concluded in favor of the topdressing application of P for better distribution in the root system (BARRETO and FERNANDES, 2002) [5] and to enlarge the availability of P in the soil, particularly in the application via fertirrigation (MAROUELLI et al., 2015) [14] an increment in P absorption by the plant does not necessarily imply in proportional productivity gains (PEREIRA et al., 2018) [19] . The application of part of the phosphate in topdressing may have favored a better distribution of the root system and thus, greater absorption of nutrients. Barreto and Fernandes (2002) [5] found greater root biomass and root distribution of maize under the effect of topdressing fertilization (broadcast) in comparison to pre-planting fertilization. The accumulations of P found in this work are generally higher than those observed by Silva et al. (2012) [22] for cv. Olimpia, 8.12 kg ha -1 or 1.58 g plant -1 P with a density of 5,144 plants ha -1 , but lower than the maximum accumulation presented by Vidigal et al. (2009) [24] from 3.62 g plant -1 (18.1 kg ha -1 for 5,000 plants ha -1 ) in cv. Crimson Sweet. However, the work of Silva et al. (2012) [22] was carried out in Eutrophic Cambisol of limestone origin using 11.6 mg dm -3 P (Mehlich-1), where a total of 220 kg ha -1 of P2O5 was applied, while that of Vidigal et al. (2003) was carried out in a sandy soil with 70.65 mg dm -3 of P (ion exchange resin), and the plants received the equivalent of 300 kg ha -1 of P2O5 in addition to organic fertilization. Differences in the accumulation of P in the literature may be the response of the genotype-environment interaction, therefore interfering in the speed of plant development and, consequently, in the potential of accumulation of nutrients. The high harvest index (between 83% and 92% -data not shown), associated to a short cycle (69 DAE, with flowering and fruiting at 28 and 38 DAE, respectively) found in this study may have impaired the balance between source and sink, in order to adjust the input of assimilates to their demand (MARSCHNER, 2012; DUARTE and PEIL, 2008) [15, 6] . Lins et al. (2013) [12] explain that the watermelon crop undergoes great changes in source-drain relations after pollination, where the fruits are the favored drains. In work using cv. Magnum in sandy soil, in Mossoró, state of Rio Grande do Norte, Pereira et al. (2018) [19] explained that the climatic conditions favored the shortening of the cycle (55 DAE, beginning of fruiting at 27 DAE) and rapid accumulation of nutrients (50% up to 2/3 of the cycle). The highest K accumulations are found in treatments F0275 (52.89 g plant -1 ), F1168 (47.17 g plant -1 ), F1397 (45.55 g plant - ) and F1275 (41.84 g plant -1 ), corresponding to values between 245 and 309 kg ha -1 K (Figure 3A-3B). Nevertheless, it should be noted that the maximum point for F1397 occurred around 58 DAE, reducing from there to approximately 31.92 g plant-1 K at 69 DAE, which is lower than that estimated for the F176 at the same period (34.56 g plant -1 ). Because K is a high mobility nutrient, this reduction can be attributed mainly to the abortion of already formed fruits. The K accumulations in this study are higher than those presented in a study developed in Cambisol Eutrophic with cv. Olímpia (5,114 plants ha -1 ), 10.30 g plant -1 (SILVA et al., 2012) [22] and in Quartzarenic Neosol with cv. Crimsom Sweet (5,000 plants ha -1 ), 24.19 g plant -1 (VIDIGAL et al., 2009) [24] . On the other hand, and Cecílio Filho (2004) [9] found a K accumulation of 79.3 g plant -1 by the hybrid Tide in a medium-textured dystrophic Red-Yellow Argisol, but with an expectation per area of 155.5 kg ha -1 of K, due to the density of planting used in the experiment (1960 plants ha -1 ). This interference of plant density on the accumulation of nutrients was also observed by Paula et al. (2011) [18] who chose to use the relationships between productivity and nutrient exports per plant instead of area unit, in a study about the nutritional requirement of N, P and K in melon and watermelon crops. At the intermediate doses of F1: F1168 and F1275 phosphate fertilizer, K accumulation rates were increasing, ranging from 0.88 to 1.38 g day -1 and from 0.43 to 1.65 g day -1 , respectively. In F0168, the K accumulation rate decreased from 1.05 to 0.54 g day -1 , between 28 and 69 DAE and in F0275, the absorption rate increased to 0.93 g day -1 at 40 DAE, reduced thereafter to 0.41 g day -1 , at 69 DAE (Figure 5E-5F). The acceleration or stabilization of K uptake rates over time should be related to better distribution of the root system, which may increase nutrient uptake efficiency to a certain extent via diffusion (MARSCHNER, 2012) [15] although K uptake via mass flow can be more representative in conditions of its high concentration in the soil solution (RUIZ et al., 1999) [20] . On the other hand, the reduction in K accumulation rates may be a consequence of the decline of nutrient uptake efficiency by the roots as the cycle advances, particularly at the beginning of the reproductive phase, where nutrient partitioning is prioritized and assimilated to the fruits, to the detriment of root growth (MARSCHNER, 2012) [15] . Regarding Ca, the following order of total accumulation was found at the 69 DAE: F0275>F1168>F1275>F176 (Figure 4A-4B). (Figure 4A-4B). Accumulation peaks of Ca ranged between 50 and 54 DAE, and an intense reduction occurred, ranging from 43% to 82% of the respective maximum (Figure 4A-4B), which should be associated with different proportions of leaf biomass caused by senescence. This is because the movement of Ca in the plant occurring mainly in the xylem, via the transpiratory current, and because of its low redistribution by the phloem (GRANGEIRO and CECÍLIO FILHO, 2004; MALAVOLTA et al., 1997; VIDIGAL et al., 2009) therefore contributing for its concentration in the leaves rather than in the fruits [9,13,24] . The maximum Ca content is higher at the greatest doses of phosphate, corresponding to 20.32 and 14.36 g plant -1 , or 118.81 and 83.96 kg ha -1 Ca, to F1397 and F0397, respectively (Figure 4A-4B), and can be explained mainly by the composition of the triple superphosphate (12% CaO). Silva et al. (2012) [22] reported a Ca maximum equivalent to 3.46 g plant -1 (17.8 kg ha -1 ) for cv. Olympia and 5.58 g plant -1 (28.7 kg ha -1 ) for cv. Leopard grown in Eutrophic Cambisol originating from the Jandaíra limestone, in Baraúna, state of Rio Grande do Norte. On the other hand, Vidigal et al. (2009) [24] in a work with the Crimson Sweet hybrid in sandy soil in the northern region of Minas Gerais, indicated a maximum Ca accumulation of 19.23 g plant -1 (96.15 kg ha -1 of Ca). It was observed in this work that the maximum accumulations of Ca between the treatments that received phosphate were between 9.71 and 22.32 g plant -1 (Figure 4A-4B). In the absence of phosphate (Adc1), the maximum Ca accumulation (6.62 g plant -1 ) (Figure 4A) corresponds between 32% and 64% of the maximum values observed for the other treatments (Figure 4A-4B) due to a smaller growth of the plant. Under these conditions, nutrient absorption is seriously impaired, particularly those that are more dependent on transpiration flow (mass flow), such as Ca. At 69 DAE, the decreasing order of the highest Mg accumulations observed was as it follows: F1168>F0275>F1275>F1397 (Figure 5A-5B). However, the highest Mg accumulations were obtained with F1397 (2.58 g plant -1 at 52 DAE), followed by F0275 (2.02 g plant -1 at 56 DAE), F0397 (1.67 g plant -1 at 51 DAE) and F1168 (1.64 g plant -1 at 69 DAE) (Figure 5A-5B). Maximum accumulation of 1.51 g plant -1 of Mg (at 57 DAE) was observed in Adc2, which is equivalent to that obtained with F0168 (56 DAE) and higher than F076 (1.28 g plant -1 at 56 DAE) and F176 (1.43 g plant -1 at 55 DAE). This can be explained by the lower K accumulation in Adc2 in relation to these treatments, therefore reducing the effect of competitive inhibition with Mg (Malavolta et al., 1997) [13] . The maximum Mg accumulation in Adc1 corresponds to only 0.75 g plant -1 (Figure 6C), or between 29% and 58% of that estimated for the other treatments. In general, the effects of treatments on the Mg uptake can be attributed mainly to plant growth, thus, reflecting the potential for nutrient accumulation. In a study with grapevines, Skinner and Mattews (1990) [23] suggested that Mg uptake would be less sensitive than its translocation in response to the P supply. The S accumulations increase until the end of the cycle, and for F0, due to the asymptotic behavior of the fertilization response, larger differences occur between the 76 and 168 kg ha -1 doses of P2O5 (Figure 6A). From the equations shown in Figures 6A and6B, it can be deduced that the F1 fertilization provided greater S accumulations for the same dose in relation to F0. For doses between 76 and 397 kg ha -1 P2O5, total accumulations were estimated from 0.88 to 1.12 g plant -1 for F1 fertilization and from 0.71 to 0.90 g plant -1 for F0 fertilization. The S accumulation in Adc2 (0.77 g plant -1 at 69 DAE) (Figure 6C) is equivalent to the 96 kg ha -1 P2O5 dose at F0 fertilization (Figure 6A), whereas, for Adc1, a model was not adjusted because of the non-significance of the F test for the unfolding as a function of time. The highest S accumulations in F1 fertilization in relation to F0 must be related to the greater P availability in the former. Kumar and Singh (1980) [11] identified positive P interaction over S uptake in a work using soybean crop. Alvarez et al. (2007) [2] reported the existence of several studies that point to a strong positive interaction between P and S, whose effects may be related to several metabolic processes in the plant and also as a result of the displacement of the adsorbed S in the soil due to P, which presents higher bonding energy. The general order of the maximum nutrient accumulation in F0 and F1 fertilizations was: K> N> Ca> P> Mg> S, except for F0275 treatment, where Mg accumulation is slightly higher than that of P. While in the additional treatments a higher Ca proportion was found by modifying the order of nutrient accumulation in Adc2 for K> Ca> N> Mg ≈ P> S. In work with cv. Magnum in sandy soil, Pereira et al. (2018) [19] found a lower P proportion in relation to Mg when applying phosphate only on pre-planting (137 kg ha-1): K> N> Ca> Mg> P> S.
Conclusions
The greatest total accumulations of P and S occur with F1 fertilization (pre-planting + fertirrigation), but in general, the characteristics evaluated in the study were dependent on the interaction between rates and manners of fertilization, where F0275 and F1168 stood out for the accumulation of other nutrients.
Figures and tables from the paper
References
23 in the original paper- Almeida EIB, Nóbrega GN, Corrêa MCM, Pinheiro EAR, ARAÚJO NA. Crescimento e marcha de absorção de micronutrientes para a cultivar de melancia Crimson Sweet. Revista Agro@mbiente On-line. 2014; 8(1):74-80.
- Alvarez VH, Roscoe R, Kurihara CH, Pereira NF et al. Enxofre. In: Novais, R. F.; Alvarez, V. H.; Barros, N. F.; Fontes, R. L.; Cantarutti, B. C.; NEVES, J. C. (Ed) Fertilidade do solo. Viçosa: Sociedade Brasileira de Ciência do Solo, 2007, 595-644.
- Alves VMC, Magalhaes JV, Vasconcellos CA, Novais RF, Bahia Filho AFC, França GE et al. Acúmulo de nitrogênio e de fósforo em plantas de milho afetadas pelo suprimento parcial de fósforo às raízes. Revista Brasileira de Ciência do Solo, Viçosa. 1999; 23(2):299305. http://dx.doi.org/10.1590/S010006831999000200014
- Araújo AP, Machado CTT. Fósforo In: Fernandes MS. (Ed.). Nutrição mineral de plantas. Viçosa: Sociedade Brasileira de Ciência do Solo, 2006, 253-280.
- Duarte TS. Peil RMN, Montezano EM. Crescimento de frutos do meloeiro sob diferentes relações fonte:dreno. Horticultura Brasileira. 2008; 26(3):342-347.
- Fernandes AM, Soratto RP. Nutrition, dry matter accumulation and partitioning and phosphorus use efficiency of potato grown at different phosphorus levels in nutrient solution. Revista Brasileira de Ciência do Solo. 2012; 36:1528-1537. http://dx.doi.org/10.1590/S0100-06832012000500017
- Ferreira DF. Sisvar versão 5.3 (Biud 75). Sistemas de análises de variância para dados balanceados: Programa de análises estatísticas e planejamento de experimentos. Lavras, Universidade Federal de Lavras, 2010.
- Grangeiro LC, Cecílio Filho AB. Acúmulo e exportação de macronutrientes pelo híbrido de melancia Tide. Horticultura Brasileira, Brasília. 2004; 22(1):9397. http://dx.doi.org/10.1590/S010205362004000100019
- Hopkins BG, Horneck DA, MacGuidwin AE. Improving phosphorus use efficiency through potato rhizosphere modification and extension. American Journal of Potato Research. 2014; 91(2):161-174. http://dx.doi.org/10.1007/s12230-014-9370-3
- Kumar V, Singh M. Sulfur, phosphorus and molybdenum interactions in relation to growth, uptake and utilization of sulfur in soybean. Soil Science. 1980; 129(5):297-304. http://dx.doi.org/10.1097/00010694198005000-00006
- Lins HA, Queiroga RCF, Pereira AM, Silva GD, Albuquerque JRT. - dreno. Revista Verde, Mossoró. 2013; 8(3):143-149.
- Malavolta Euripedes VITTI, Godofredo Cesar OLIVEIRA, Sebastião Alberto. Avaliação do estado nutricional das plantas: princípios e aplicações. 2. ed. Piracicaba: POTAFOS, 1997, 201.
- Marouelli WA, Guimaraes TG, Braga MB, Carvalho WL. Frações ótimas da adubação com fósforo no pré-plantio e na fertirrigação por gotejamento de tomateiro. Pesquisa Agropecuária Brasileira. 2015; 50(10):949-957. http://dx.doi.org/10.1590/S0100204X2015001000011
- Marschner Horst. Mineral nutrition of higher plants. 3. Ed. London: Elsevier, 2012, 643.
- Merriam John L, Keller Jack. Farm irrigation system evaluation: a guide for management. Logan: Utah State University, 1978, 271.
- Mohammad MJ, Hammouri A, Ferdows AE. Phosphorus fertigation and preplant conventional soil application of drip irrigated summer squash. Journal of Agronomy. 2004; 3(3):162-169.
- Paula JAA, Medeiros JF, Miranda NO, Oliveira FA, Lima CJGS. Metodologia para determinação das necessidades nutricionais de melão e melancia. Revista Brasileira de Engenharia Agrícola e Ambiental, Campina Grande. 2011; 15:911-916.
- Pereira NS, Alves Júnior AR, Celedônio WF, Rodrigues EA, Chaves SWP, Medeiros JF et al. Phosphate fertilization influences macronutrient accumulation in watermelon cv Magnum. Horticultura Brasileira. 2018; 36(3):346-352. http://dx.doi.org/10.1590/s0102-053620180310
- Ruiz HA, Miranda JE, Conceição JCS. K, Ca, Mg às plantas de arroz. Revista Brasileira da Ciência do Solo, Viçosa. 1999; 23(4):1015-1018. http://dx.doi.org/10.1590/S010006831999000400029
- Silva Fábi Cesar. Manual de análises químicas de solos, plantas e fertilizantes. 2 ed. Brasília: Embrapa Informação Tecnológica, 2009, 627.
- Silva MVT, Chaves SWP, Medeiros JF, Souza MS, Santos APF, Oliveira FL et al. Acúmulo e exportação de macronutrientes em melancieiras fertirrigadas sob ótimas condições de adubação nitrogenada e fosfatada. CSA -Agropecuária Científica no Semi-Árido. 2012; 98(4):55-59.
- Skinner PW, Matthews MAA. Novel interaction of magnesium translocation with the supply of phosphorous to root of grapevine (Vitis vinifera L.). Plant, Cell and Environment, Oxford. 1990; 13(8):821826. https://doi.org/10.1111/j.13653040.1990.tb01098.x
- Vidigal SM, Pacheco DD, Costa EL, Facion CE. Crescimento e acúmulo de macro e micronutrientes pela melancia em solo arenoso. Revista Ceres. 2009; 56(1):112-118.